Movie
 Controller


[English] 日本語
 Yorodumi
- PDB-9t64: Cytoplasmic lattice filament repeat unit with the central FBXW-SK... -
+ Open data

- Basic information
| Entry | Database: PDB / ID: 9t64 | |||||||||||||||||||||||||||||||||
|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|
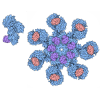
| Title | Cytoplasmic lattice filament repeat unit with the central FBXW-SKP1 complex | |||||||||||||||||||||||||||||||||
 Components |
| |||||||||||||||||||||||||||||||||
 Keywords | UNKNOWN FUNCTION / Ubiquitination / Complex / Filament | |||||||||||||||||||||||||||||||||
| Function / homology |  Function and homology information regulation of translation by machinery localization / cytoplasm organization / ooplasm / Signaling by BMP / Prolactin receptor signaling / embryonic process involved in female pregnancy / establishment of organelle localization / Microtubule-dependent trafficking of connexons from Golgi to the plasma membrane / Cargo trafficking to the periciliary membrane / Sealing of the nuclear envelope (NE) by ESCRT-III ...regulation of translation by machinery localization / cytoplasm organization / ooplasm / Signaling by BMP / Prolactin receptor signaling / embryonic process involved in female pregnancy / establishment of organelle localization / Microtubule-dependent trafficking of connexons from Golgi to the plasma membrane / Cargo trafficking to the periciliary membrane / Sealing of the nuclear envelope (NE) by ESCRT-III / cortical granule exocytosis / establishment or maintenance of apical/basal cell polarity / subcortical maternal complex / endoplasmic reticulum localization / Chromatin modifying enzymes / protein storage / structural constituent of cytoplasmic lattice / cytoplasmic lattice / Carboxyterminal post-translational modifications of tubulin / Intraflagellar transport / COPI-independent Golgi-to-ER retrograde traffic / SCF-beta-TrCP mediated degradation of Emi1 / HSP90 chaperone cycle for steroid hormone receptors (SHR) in the presence of ligand / E3 ubiquitin ligases ubiquitinate target proteins / Downregulation of SMAD2/3:SMAD4 transcriptional activity / ZNF598 and the Ribosome-associated Quality Trigger (RQT) complex dissociate a ribosome stalled on a no-go mRNA / histone H3K18 ubiquitin ligase activity / histone H3 ubiquitin ligase activity / Regulation of BACH1 activity / histone H3K14 ubiquitin ligase activity / spermatogonial cell division / histone H3K23 ubiquitin ligase activity / COPI-mediated anterograde transport / PINK1-PRKN Mediated Mitophagy / Inactivation of CSF3 (G-CSF) signaling / SCF(Skp2)-mediated degradation of p27/p21 / Regulation of TNFR1 signaling / MAP3K8 (TPL2)-dependent MAPK1/3 activation / Kinesins / histone H3 reader activity / Regulation of RUNX2 expression and activity / Degradation of GLI1 by the proteasome / GSK3B-mediated proteasomal degradation of PD-L1(CD274) / Cyclin D associated events in G1 / FBXL7 down-regulates AURKA during mitotic entry and in early mitosis / IKK complex recruitment mediated by RIP1 / fertilization / Orc1 removal from chromatin / GSK3B and BTRC:CUL1-mediated-degradation of NFE2L2 / Dectin-1 mediated noncanonical NF-kB signaling / NIK-->noncanonical NF-kB signaling / cortical granule / PKR-mediated signaling / regulation of establishment of protein localization / RHO GTPases activate IQGAPs / Aggrephagy / Oxygen-dependent proline hydroxylation of Hypoxia-inducible Factor Alpha / Mitotic Prometaphase / EML4 and NUDC in mitotic spindle formation / Resolution of Sister Chromatid Cohesion / COPI-dependent Golgi-to-ER retrograde traffic / Degradation of beta-catenin by the destruction complex / Activation of NF-kappaB in B cells / apical cortex / Recycling pathway of L1 / Iron uptake and transport / positive regulation of meiotic nuclear division / The role of GTSE1 in G2/M progression after G2 checkpoint / chromosomal DNA methylation maintenance following DNA replication / regulation of RNA stability / embryonic cleavage / positive regulation of embryonic development / intermediate filament cytoskeleton / axonemal microtubule / CLEC7A (Dectin-1) signaling / Interleukin-1 signaling / FCERI mediated NF-kB activation / Hedgehog 'off' state / RHO GTPases Activate Formins / F-box domain binding / Loss of Nlp from mitotic centrosomes / Recruitment of mitotic centrosome proteins and complexes / Loss of proteins required for interphase microtubule organization from the centrosome / Anchoring of the basal body to the plasma membrane / Recruitment of NuMA to mitotic centrosomes / AURKA Activation by TPX2 / Separation of Sister Chromatids / Downstream TCR signaling / hemi-methylated DNA-binding / Peroxisomal protein import / GLI3 is processed to GLI3R by the proteasome / embryonic pattern specification / Regulation of PLK1 Activity at G2/M Transition / Ubiquitin-Mediated Degradation of Phosphorylated Cdc25A / regulation of epithelial cell proliferation / PcG protein complex / Neddylation / MHC class II antigen presentation / gap junction / establishment of spindle localization Similarity search - Function | |||||||||||||||||||||||||||||||||
| Biological species |   Mus musculus (house mouse) | |||||||||||||||||||||||||||||||||
| Method | ELECTRON MICROSCOPY / subtomogram averaging / cryo EM / Resolution: 7.3 Å | |||||||||||||||||||||||||||||||||
 Authors | Singh, K. / Harasimov, K. / Carter, A.P. | |||||||||||||||||||||||||||||||||
| Funding support |  United Kingdom, European Union, 3items
| |||||||||||||||||||||||||||||||||
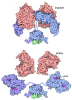
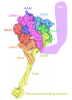
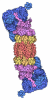
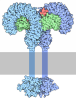
 Citation | Journal: EMBO J / Year: 2026 Title: In-situ cryo-ET of mouse embryos reveals cytoplasmic lattices contain ubiquitin-charged E2-E3 ligase assemblies. Authors: Kashish Singh / Katarina Harasimov / Kathy K Niakan / Andrew P Carter / Abstract: Cytoplasmic lattices (CPLs) are filamentous assemblies essential for mammalian embryonic development. They are known to regulate organelle organization, spindle assembly, and protein homeostasis, but ...Cytoplasmic lattices (CPLs) are filamentous assemblies essential for mammalian embryonic development. They are known to regulate organelle organization, spindle assembly, and protein homeostasis, but their molecular functions remain unclear. Here, we develop a strategy combining cryo-focused ion beam milling and cryo-electron tomography to resolve macromolecular complexes directly in mammalian embryos. Using this approach, we determine the in situ structure of cytoplasmic lattices within 6/8-cell mouse embryos at ~4.7 Å resolution. CPL filaments are built from multiple copies of at least fourteen proteins arranged into a ~4.5 MDa repeating unit. The repeat contains a central cavity that is open at the back and lined with multiple FBXW-SKP1 complexes and three modules, each containing the E2 ubiquitin-conjugating enzyme UBE2D and the E3 ligase UHRF1. We resolve two CPL states: one is consistent with a ubiquitin-charged UBE2D, where ubiquitin is held in an open, inactive conformation by binding the scaffold protein PADI6; the second lacks discernible ubiquitin density and shows structural changes compatible with ubiquitin becoming available for transfer. Our findings support a model in which CPLs function as large ubiquitin ligase assemblies during early embryonic development. | |||||||||||||||||||||||||||||||||
| History |
|
- Structure visualization
| Structure viewer | Molecule: MolmilJmol/JSmol |
|---|
- Downloads & links
-Download
| PDBx/mmCIF format | 9t64.cif.gz | 4.8 MB | Display | PDBx/mmCIF format |
|---|---|---|---|---|
| PDB format | pdb9t64.ent.gz | Display | PDB format | |
| PDBx/mmJSON format | 9t64.json.gz | Tree view | PDBx/mmJSON format | |
| Others |  Other downloads |
-Validation report
| Arichive directory | https://data.pdbj.org/pub/pdb/validation_reports/t6/9t64ftp://data.pdbj.org/pub/pdb/validation_reports/t6/9t64 | HTTPS FTP |
|---|
-Related structure data
| Related structure data |  55604MC  9t63C  9t65C  9t66C  9t67C  9t68C M: map data used to model this data C: citing same article ( |
|---|---|
| Similar structure data |


-Links
 PDBj
- Assembly
| Deposited unit | 
|
|---|---|
| 1 |
|
-Components
-Protein , 12 types, 62 molecules 0S123ABCDEFGHIJKLmstuvwxyz58NQ...
| #1: Protein | Mass: 48055.301 Da / Num. of mol.: 2 / Source method: isolated from a natural source / Source: (natural) Mus musculus (house mouse) / References: UniProt: Q9CWU5#2: Protein | Mass: 76854.109 Da / Num. of mol.: 24 / Source method: isolated from a natural source / Source: (natural) Mus musculus (house mouse) / References: UniProt: Q8K3V4#4: Protein | Mass: 65187.332 Da / Num. of mol.: 4 / Source method: isolated from a natural source / Source: (natural) Mus musculus (house mouse) / References: UniProt: Q9WVB3#5: Protein | Mass: 18481.295 Da / Num. of mol.: 4 / Source method: isolated from a natural source / Source: (natural) Mus musculus (house mouse) / References: UniProt: Q9CWE6#6: Protein | Mass: 25643.373 Da / Num. of mol.: 2 / Source method: isolated from a natural source / Source: (natural) Mus musculus (house mouse) / References: UniProt: Q9D0L1#7: Protein | Mass: 108001.281 Da / Num. of mol.: 4 / Source method: isolated from a natural source / Source: (natural) Mus musculus (house mouse) / References: UniProt: L7N1W9#9: Protein | Mass: 88436.805 Da / Num. of mol.: 3 / Source method: isolated from a natural source / Source: (natural) Mus musculus (house mouse)References: UniProt: Q8VDF2, RING-type E3 ubiquitin transferase #10: Protein | Mass: 16706.133 Da / Num. of mol.: 3 / Source method: isolated from a natural source / Source: (natural) Mus musculus (house mouse)References: UniProt: P61079, E2 ubiquitin-conjugating enzyme, (E3-independent) E2 ubiquitin-conjugating enzyme #11: Protein | Mass: 49962.172 Da / Num. of mol.: 3 / Source method: isolated from a natural source / Source: (natural) Mus musculus (house mouse)References: UniProt: P68373, Hydrolases; Acting on acid anhydrides; Acting on GTP to facilitate cellular and subcellular movement #12: Protein | Mass: 49877.824 Da / Num. of mol.: 3 / Source method: isolated from a natural source / Source: (natural) Mus musculus (house mouse) / References: UniProt: P68372#13: Protein | Mass: 39676.895 Da / Num. of mol.: 5 / Source method: isolated from a natural source / Source: (natural) Mus musculus (house mouse)#14: Protein | Mass: 18693.992 Da / Num. of mol.: 5 / Source method: isolated from a natural source / Source: (natural) Mus musculus (house mouse) / References: UniProt: Q9WTX5 |
|---|
-NACHT, LRR and PYD domains-containing protein ... , 2 types, 7 molecules 47MPAGZn
| #3: Protein | Mass: 131468.547 Da / Num. of mol.: 4 / Source method: isolated from a natural source / Source: (natural) Mus musculus (house mouse) / References: UniProt: Q9R1M5#8: Protein | Mass: 113527.188 Da / Num. of mol.: 3 / Source method: isolated from a natural source / Source: (natural) Mus musculus (house mouse) / References: UniProt: Q6B966 |
|---|
-Details
| Has protein modification | N |
|---|
-Experimental details
-Experiment
| Experiment | Method: ELECTRON MICROSCOPY |
|---|---|
| EM experiment | Aggregation state: FILAMENT / 3D reconstruction method: subtomogram averaging |
- Sample preparation
| Component | Name: Multi-subunit complex of the cytoplasmic lattice filament repeat unit Type: COMPLEX / Entity ID: all / Source: NATURAL |
|---|---|
| Source (natural) | Organism: Mus musculus (house mouse) |
| Buffer solution | pH: 7.5 |
| Specimen | Embedding applied: NO / Shadowing applied: NO / Staining applied: NO / Vitrification applied: YES |
| Vitrification | Cryogen name: ETHANE |
- Electron microscopy imaging
| Experimental equipment |  Model: Titan Krios / Image courtesy: FEI Company |
|---|---|
| Microscopy | Model: TFS KRIOS |
| Electron gun | Electron source:  FIELD EMISSION GUN / Accelerating voltage: 300 kV / Illumination mode: FLOOD BEAM |
| Electron lens | Mode: BRIGHT FIELD / Nominal defocus max: 4000 nm / Nominal defocus min: 1000 nm |
| Image recording | Electron dose: 3.5 e/Å2 / Avg electron dose per subtomogram: 115 e/Å2 / Film or detector model: FEI FALCON IV (4k x 4k) |
- Processing
| EM software |
| ||||||||||||
|---|---|---|---|---|---|---|---|---|---|---|---|---|---|
| CTF correction | Type: PHASE FLIPPING AND AMPLITUDE CORRECTION | ||||||||||||
| Symmetry | Point symmetry: C1 (asymmetric) | ||||||||||||
| 3D reconstruction | Resolution: 7.3 Å / Resolution method: FSC 0.143 CUT-OFF / Num. of particles: 34451 / Symmetry type: POINT | ||||||||||||
| EM volume selection | Num. of tomograms: 1153 / Num. of volumes extracted: 134387 |